 2026, Vol. 56


2. 中国海洋大学山东省海水绿色养殖与智慧渔业重点实验室, 山东 青岛 266003;
3. 中国海洋大学未来海洋学院, 山东 青岛 266100
潮间带是海陆交界的过渡区域,其环境动态受到潮汐周期性涨落的影响,时空异质性显著。在岩相潮间带,温度等环境因子变化剧烈,形成周期性交替的极端环境[1-2]。为适应这种持续的环境胁迫,岩相潮间带的底栖动物演化出独特的生态适应策略,以维系群落结构稳定性和物种多样性[3]。
青岛岩相潮间带底质结构多样、潮汐梯度明显,为独特而多样的底栖生物群落提供了良好的生存与繁衍条件,形成了具有区域特色的潮间带生态系统[4]。自20世纪30年代起,青岛地区已开展多次大型底栖动物调查,并陆续进行过多次系统性研究[5-7],但仍存在以下不足:首先,已有调查多基于单次或季节性采样,难以完整捕捉群落结构的月度动态变化;其次,对不同潮位高度生物群落结构的量化比较仍较为薄弱;此外,结合高分辨率环境因子开展“环境-群落”耦合关系的研究尚存空白,导致难以精准量化关键环境因子对底栖生物群落的调控作用。
为填补上述研究空白,本研究在青岛岩相潮间带开展了为期12个月的月度生态调查,系统研究了高、中潮位大型底栖动物群落的组成与分布特征,旨在量化其群落结构的时空动态;并结合温度、盐度、叶绿素a等关键环境因子,解析环境对群落结构变化的驱动机制与相对贡献。研究成果将深化对潮间带生物群落动态变化规律的理解,有望为温带岩相潮间带的生态保护与管理提供理论支撑。
1 材料与方法青岛市地处山东半岛南端,位于黄渤海交汇处,属典型海洋性季风气候,四季分明、气温适中,这为潮间带生态系统稳定和海洋生物多样性维持提供了良好条件。本研究调查区位于青岛市汇泉角(36.047 6°N, 120.346 4°E),地处太平湾与汇泉湾交汇带,具有典型的海蚀岩岸特征(见图 1)。该区域以裸露花岗岩礁石为主,整体呈东北-西南走向,低潮时礁体延伸入海[8]。复杂的水动力环境与岩质基底共同塑造了丰富的底栖动物类群。

|
(左图为区位索引图,来源于山东省自然资源厅监制标准地图(审图号: 鲁SG(2025)084号), 黑色框标示出本研究区域的位置。The left image is the location index map, sourced from the standard map supervised by the Department of Natural Resources of Shandong Province (map review number: SG(2025)084), with the location of the research area indicated by a black box. ) 图 1 调查区域地理位置图 Fig. 1 Geographic location of the survey area |
本研究时间为2023年9月至2024年8月,每月大潮日低潮时段在同一区域开展生态调查,共计12次。每次调查均包括样方调查(Quadrat survey)与打点调查(Point-contact survey),并参照潮间带生态调查标准[9],结合当地地貌特点进行适当调整。调查对象为体长大于0.5 mm的底栖动物,主要包括腹足纲(Gastropoda)、双壳纲(Bivalvia)、多板纲(Polyplacophora)和鞘甲纲(Thecostraca)等类群,这些类群在岩相潮间带中具有高度代表性与生态指示意义[10]。
1.1 抛框调查方法本研究在选定的岩相潮间带,于高潮位最高处设置了一条30 m长的固定基线。沿基线每隔3 m设置1条垂直于海岸线的样线,11条样线共界定出10个样面。根据生物分布特征,将每个样面划分为高潮位和中潮位(本次调查不涉及低潮位)。界限依据局部物种分布划分:中潮位为牡蛎与藤壶共存区,高潮位则为藤壶分布带上缘以上区域[6, 11]。每个样面在高潮位设置1个、中潮位设置2个样方框,总计30个调查样本,在每个样本内随机抛掷0.5 m×0.5 m样方框,记录框内所有体长大于0.5 mm的大型底栖动物的种类和数量。物种鉴定参考《中国水生贝类图谱》《胶州湾大型底栖生物鉴定图谱》《中国近海底栖动物分类体系》和WoRMS网站[12-15]。将调查记录整理并换算为密度数据,用于后续统计分析。
1.2 打点调查方法打点调查在布设的11条样线上进行。沿每条样线从基线起每隔30 cm设置一个标记点,以确保标记点的均匀分布与代表性。在每个标记点,记录其半径15 cm范围内距离最近且不重复的3个物种。若该范围内物种不足3个,则用“NA”记录空缺。将调查记录整理为沿样线纵向的物种出现数据,用于潮位划分;并将各样线的物种出现情况转化为定性数据,用于后续物种数统计分析。
1.3 环境因子数据获取与处理从欧洲中期天气预报中心第五代全球气候再分析数据集ERA5每小时单层数据中获取了分辨率为0.25°×0.25°的2 m气温(2 m air temperatures, 2 m T)、海表温度(Sea surface temperatures, SST)和总降水量(Total precipitation, Precip.)[16]。从哥白尼网站(Copernicus-Global Ocean Biogeochemistry Hindcast, Global Ocean Physics Reanalysis)获取了分辨率为1/12(°)×1/12(°)的每小时海水盐度(Sea water salinity, SSS),以及分辨率为0.25°×0.25°的每日海水叶绿素a的浓度(Mass concentration of chlorophyll a, Chl a)[17-18]。所有环境因子均经计算转换为日均值,并用于后续的环境关联分析。
1.4 数据分析 1.4.1 优势度分析对抛框调查数据进行整理,计算每个月份各潮位的优势度指数(Y)。计算公式如下:
| $ {Y_i} = ({n_i}/N) \times {f_i}。$ | (1) |
式中:ni指的是第i种大型底栖动物的个体数; N为样品的总个体数;fi为第i种大型底栖动物在该框出现的频率,即该物种出现的样方数与样品总样方数的比值。当该种优势度Yi>0.02时,则该种为该潮位的优势种[19]。
1.4.2 多样性分析物种数多样性分析采用打点调查数据,其余多样性分析采用抛框调查数据。物种数多样性分析以每条样线的物种数为一个样本点。月份多样性分析以每个样面(从高到低3个样本框)作为一个样本点,潮高多样性分析将每个断面每个潮位作为一个样本点。用Shannon-Wiener多样性指数(H′)表征群落的多样性水平[20];用Pielou均匀度指数(J′)评估群落的均匀度[21],用Margalef丰富度指数(D)反映群落的物种丰富度[22]。各指数的计算公式如下:
| $ H' =- \sum\limits_{i = 1}^S {{p_i}{\rm{ln}}{p_i}} ,$ | (2) |
| $ \begin{array}{*{20}{l}} {J' = H'/{\rm{ln}}S} \end{array},$ | (3) |
| $ {D = (S- 1)/{\rm{ln}}N}。$ | (i) |
公式(2)—(4)中:S是大型底栖动物总物种数;N是大型底栖动物总个体数;pi是第i种大型底栖动物的个体数与总个体数N的比值。
不同潮位间多样性指数的差异采用Wilcoxon秩和检验进行分析。采用ggplot2与gghalves包绘图[23-24],可视化不同月份间物种数量、H′、J′和D的分布特征。
1.4.3 排序与群落结构差异分析采用R语言vegan包,基于Jaccard距离对不同月份和不同潮位的物种组成数据进行非度量多维标度分析(Non-metric multidimensional scaling,NMDS),以反映样本间群落结构差异[25-26]。以stress值评估排序结果,当stress<0.20时,指示排序结果具有较好的可解释性[27-28]。不同分组间群落结构差异采用置换多元方差分析(Permutational multivariate analysis of variance,PERMANOVA)检验,组内离散度差异采用置换多元离散度检验(Permutational analysis of multivariate dispersions,PERMDISP)评估。同时对NMDS1和NMDS2轴采用Kruskal-Wallis检验进行辅助分析。
1.4.4 环境因子关联分析使用vegan包中的Hellinger方法对物种丰度数据进行标准化处理。结合标准化后的环境数据,采用Bray-Curtis距离度量样本间物种组成的相似性,并进一步利用microeco包进行基于距离的冗余分析(Distance-based redundancy analysis,dbRDA),以评估环境因子对物种丰度的影响[29]。在dbRDA分析中,环境因子的贡献通过排序图直观展示,同时将结果按季节分组呈现(秋:9—11月;冬:12月—次年2月;春:3—5月;夏:6—8月)。采用Pearson相关系数检验分析各目级分类单元丰度与环境变量之间的相关性。
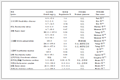
2 结果 2.1 大型底栖动物种类组成与物种数变化本研究共鉴定出大型底栖动物19种,隶属2门、4纲、9目、14科(见表 1)。东方小藤壶(Chthamalus challengeri)、粒结节滨螺(Echinolittorina radiata)、短滨螺(Littorina brevicula)、长牡蛎(Crassostrea gigas)、黑荞麦蛤(Xenostrobus atratus)、矮拟帽贝(Patelloida pygmaea)、嫁(Cellana toreuma)、疣荔枝螺(Thais clavigera)、紫贻贝(Mytilus galloprovincialis)、齿舌新笠贝(Nipponacmea radula)和红条毛肤石鳖(Acanthochitona rubrolineata)11个物种在每月调查中均有记录。从月度变化来看,物种数存在波动,整体呈现秋冬季节较低、春夏季节回升并趋于稳定的趋势(见图 2)。其中,3月样线平均物种数最少(8种);6月达到峰值(12种)。
|
表 1 青岛岩相潮间带大型底栖动物调查物种名录 Table 1 List of macrobenthic species surveyed in the rocky intertidal zone of Qingdao |

|
(每个散点表示对应月份中打点调查单个样线物种数。图中星号表示组间α多样性指数差异的显著性水平, *:P<0.05,**:P<0.01,***:P<0.001。Each dot represents the species richness recorded for a single transect in the corresponding month based on the point-contact survey. Asterisks indicate significant differences in alpha diversity index between groups, *: P < 0.05, **: P < 0.01, ***: P < 0.001. ) 图 2 青岛岩相潮间带大型底栖动物物种数月度变化 Fig. 2 Monthly variation in species richness of macrobenthic fauna on the rocky shore in Qingdao |
基于青岛岩相潮间带不同潮位和月份的样方调查结果,大型底栖动物的物种优势度发生了一定变化(见表 2)。整体而言,各物种的优势度指数波动较大(2.16%~99.77%),且优势种的组成呈现季节动态和潮位间异质性。优势种主要包括东方小藤壶、粒结节滨螺、短滨螺和长牡蛎。具体来看,东方小藤壶在中潮位的优势度普遍较高(57.59%~92.65%),为中潮位的绝对优势种;粒结节滨螺在所有月份的高潮位均占据显著数量优势(22.36%~99.77%),且几乎不分布于中潮位。此外,短滨螺在部分月份的高潮位中占据一定数量优势,尤其以9—11月为著;而长牡蛎在9月中潮位占据一定数量优势,其余物种在数量上均未表现出明显优势。
|
|
表 2 大型底栖动物主要优势种及优势度 Table 2 Dominant macrobenthic species and their dominance |
本研究调查区域内不同月份的多样性指数(H′)、均匀度指数(J′)和丰富度指数(D)结果如图 3所示。整体来看,H′和J′全年均处于较低水平。其中,H′在9月(0.67)和10月(0.51)相对较高;J′同样在9月(0.33)和10月(0.25)略高于其他月份,表明这两个月物种组成相对丰富且分布较为均匀。相比之下,D呈现出规律的月度变化趋势,表现为秋、冬季节下降,春、夏季节上升;在1月(冬)降至最低(0.56),随后逐步上升,至8月(夏季)达到峰值(0.98)。

|
(每个散点表示对应月份单个样面的多样性指数,该指数由该样面纵向3个样方(高潮位1个、中潮位2个)的平均密度计算所得。图中星号表示组间α多样性指数差异的显著性水平,*:P<0.05,**:P<0.01,***:P<0.001。Each dot represents the diversity index for a single plot in the corresponding month, calculated from the mean density of three longitudinal quadrats (one at high tidal level and two at middle tidal level) within that plot. Asterisks indicate significant differences in alpha diversity index between groups, *: P < 0.05, ** : P < 0.01, *** : P < 0.001. ) 图 3 大型底栖动物群落的月度多样性指数 Fig. 3 Diversity index of intertidal macrobenthic communities across months |
基于物种组成进行的非度量多维尺度分析(NMDS)结果如图 4和表 3所示,应力值(Stress)为0.144,小于阈值0.200,表明二维空间较好地反映了原始数据的相似性结构。在NMDS1维度上,不同月份之间存在差异显著(P<0.05)。1—3月NMDS1坐标值整体较高,3月后逐渐下降,至8月再次回升,呈现明显的周期性波动。而在NMDS2维度上,各月份间的差异未达到显著性(P>0.05)。

|
(星号表示不同箱线图数据组间差异的显著性水平,***:P<0.001;ns表示无显著差异,P≥0.05。Asterisks indicate significant differences between groups in the boxplot data, *** : P < 0.001; ns indicates no significant difference, P≥0.05. ) 图 4 大型底栖动物群落的月度非度量多维标度(NMDS)排序分析结果 Fig. 4 Non-metric multidimensional scaling (NMDS) ordination of macrobenthic communities across different months |
|
|
表 3 大型底栖动物群落结构月度差异的统计检验结果 Table 3 Statistical test results for monthly differences in macrobenthic community structure |
主要大型底栖动物在各月份的相对丰度如图 5所示。从物种水平看,东方小藤壶的相对丰度显著高于其他物种,月均密度均超过103 ind./m2,自成一簇;黑荞麦蛤、长牡蛎、粒结节滨螺、矮拟帽贝和短滨螺的月均密度均大于10 ind./m2,构成第二簇;其余物种丰度相对较低(月均密度<10 ind./m2),聚为第三簇。

|
图 5 大型底栖动物相对丰度的月度聚类热图 Fig. 5 Relative abundance heatmap of macrobenthic fauna across different months |
从时间维度看,月份间可依据相对丰度高低聚为两簇。3—8月物种相对丰度较高,聚成一簇;9月至次年2月物种相对丰度普遍较低,聚为另一簇。在低丰度簇中,9月的物种丰度相对均匀,与其他低丰度月份略有差异。
2.4 群落结构的潮区变化趋势 2.4.1 多样性的潮区差异不同潮位间的多样性指数(H′、J′和D)均存在极显著差异(见图 6)。高潮位的多样性指数(H′)显著低于中潮位(均值分别为0.13和0.35,P<0.001),表明中潮位具有更高的物种多样性。高潮位的丰富度指数(D)显著低于中潮位(均值分别为0.11和0.58,P<0.001),表明中潮位具有更高的物种丰富度。此外,高潮位的均匀度指数(J′)显著高于中潮位(均值分别为0.41和0.23,P<0.05),说明高潮位的物种分布更为均匀。

|
( H:高潮位,M:中潮位。图中星号表示组间α多样性指数差异的显著性水平,*:P<0.05,***:P<0.001。H: High tidal level; M: Middle tidal level. Asterisks indicate significant differences in alpha diversity index between groups, * : P < 0.05, *** : P < 0.001. ) 图 6 大型底栖动物群落的潮位多样性指数 Fig. 6 Diversity index of intertidal macrobenthic communities across tidal levels |
基于群落组成的NMDS分析显示,不同潮位在二维排序空间中呈现明显分裂,模型拟合良好(Stress=0.074)(见图 7和表 4)。在NMDS1水平上差异显著(P<0.05)。高潮位的样本点主要分布于右下方,分布较为聚集;中潮位的样本点集中于中心区域,分布较为分散。置换多元方差分析结果表明,潮位对群落组成差异具有显著影响(F=138.600,R2=0.296,P<0.001)。置换多元离散度检验结果表明,高潮位和中潮位的组内变异同样存在显著差异(F=49.678,P<0.001),其中,中潮位的离散度较大。

|
( H:高潮位,M:中潮位。星号表示不同潮位箱线图数据组间差异的显著性水平, ***: P<0.001。H: High tidal level; M: Middle tidal level. Asterisks indicate significant differences between the groups at different tidal levels, *** : P < 0.001. ) 图 7 大型底栖动物群落不同潮位的NMDS排序分析结果 Fig. 7 NMDS ordination of macrobenthic communities across different tidal levels |
|
|
表 4 大型底栖动物群落结构潮位差异的统计检验结果 Table 4 Statistical test results for tidal level differences in macrobenthic community structure |
表 5展示了调查期间不同月份环境因子的数据特征,dbRDA分析结果前两轴累计解释了不同季节环境因子对群落结构变异的85.9%(见图 8)。在环境因子中,温度相关参数(2 m T和SST)对群落结构的影响最为突出,与叶绿素(Chl a)共同构成了dbRDA1轴的主要驱动因素,三者均与夏、秋季节呈正相关,与春、冬季节呈负相关。此外,总降水量(Precip.)与盐度(SSS)也对群落季节分化具有重要贡献。降水量与夏季正相关,与冬季样本呈负相关;SSS则与春季样本正相关,与秋季样本负相关。
|
|
表 5 调查期间不同月份环境因子数据 Table 5 Monthly variation in environmental variables during the survey period |

|
( 2 m T:2 m气温;SST:海表温度;SSS:海水盐度;Precip.:总降水量;Chl a:叶绿素a浓度。2 m T: 2 m air temperature; SST: Sea surface temperature; SSS: Sea water salinity; Precip.: Total precipitation; Chl a: Mass concentration of chlorophyll a. ) 图 8 大型底栖动物群落与环境变量的dbRDA排序图 Fig. 8 dbRDA ordination of macrobenthic communities constrained by environmental variables |
用Pearson相关性检验各目级分类单元丰度与环境变量之间的相关性(见图 9)。温度相关参数(2 m T和SST)与大型底栖动物的相关性最强,其中与马蹄螺目(Trochida)和新腹足目(Neogastropoda)呈极显著正相关(P<0.001),与贻贝目(Mytilida)和藤壶目(Balanomorpha)呈极显著负相关(P<0.001)。Chl a与马蹄螺目(Trochida)和新腹足目(Neogastropoda)呈显著正相关(P<0.05),与贻贝目(Mytilida)呈显著负相关(P<0.05)。

|
( 2 m T:2 m气温;SST:海表温度;SSS:海水盐度;Precip.:总降水量;Chl a:叶绿素a浓度。星号表示环境因子与物种丰度相关性的显著性水平,*:P<0.05,**:P<0.01,***:P<0.001。2 m T: 2 m air temperature; SST: Sea surface temperature; SSS: Sea water salinity; Precip.: Total precipitation; Chl a: Mass concentration of chlorophyll a. Asterisks indicate the significance levels of correlations between environmental factors and species abundance, * : P < 0.05, **: P < 0.01, ***: P < 0.001. ) 图 9 大型底栖动物各目级分类单位与环境因子的关系 Fig. 9 Relationship between environmental variables and order-level taxa of macrobenthic fauna |
青岛岩相潮间带大型底栖动物群落结构显现明显的季节性波动。月度物种数和丰富度指数在秋、冬季节逐渐下降,于冬季达到最低,随后在春、夏季回升并于夏季达到峰值,二者变化趋势高度一致。这一季节性变化趋势暗示,秋、冬季的低温与资源匮乏等环境压力可能抑制了大型底栖动物群落的维持和恢复[30]。气温变化拐点与群落结构变化拐点基本一致,进一步支持了这一季节性环境驱动的作用。
冬季低温导致生物代谢减缓,食物供应减少,限制了多数物种的生长和繁殖。而在春、夏季,随着气温回升和初级生产力增强,底栖动物获得了更丰富的食物资源与更适宜的繁殖条件,物种数量得以恢复,群落结构逐步重建。东方小藤壶[31]、长牡蛎[32]、黑荞麦蛤[33]和紫贻贝[34]等类群在春、夏季进入孵化期或幼体附着窗口期,新个体的补充显著促进了物种丰富度的提升。此外,部分物种(如疣荔枝螺[35-36])在冬季可能进入滞育状态或向潮下带迁移,进一步影响了潮间带群落的物种丰度。值得注意的是,短滨螺[37]、矮拟帽贝[38]和嫁[39]等类群在秋、冬季仍保持一定的数量优势,反映出这些物种对低温环境的生理与行为适应能力。综上,青岛典型岩相潮间带大型底栖生物群落呈现“春夏高、秋冬低”的典型季节模式,与在东海、黄海及黄渤海等其他区域岩相潮间带观察到的季节波动模式一致,表明该季节规律在区域尺度上具有普遍性[40-43]。
3.2 潮间带垂直分带及其群落结构差异本研究表明,青岛岩相潮间带的大型底栖动物群落在垂直方向上存在显著的分带现象,不同潮区的群落结构差异显著。该区域的纵向生态格局符合典型的“滨螺带-藤壶牡蛎带-海藻带”三分模式[44],这种生态分层主要源于不同潮位区域环境因子的梯度变化。
高潮位每日仅在高潮时被海水短暂淹没,大部分时间暴露在空气中,日照强烈、温度波动剧烈、湿度低。高潮位恶劣的环境条件塑造了以粒结节滨螺和短滨螺为优势种的群落结构,这些物种普遍具有强耐旱和耐高温能力。尽管高潮位的物种多样性和群落丰富度低,但由于物种数量稀少,形成了群落均匀度相对较高的生态格局。相比之下,中潮位环境条件相对温和稳定,干湿交替规律明显,资源更为丰富。东方小藤壶和长牡蛎在中潮位全年广泛覆盖并占绝对优势,短滨螺、黑荞麦蛤和矮拟帽贝等物种具有较高丰度。得益于适宜的环境条件,中潮位的物种多样性、群落丰度及群落复杂性均显著高于高潮带,从而支撑了更高的生物多样性。
相比之下,本研究中甲壳动物等类群记录种数相对较少,可能与局地环境变化、微生境差异及人为干扰有关;同时,也可能受到本研究调查范围和潮位覆盖程度的影响,尤其是低潮位样带覆盖不足,可能使部分主要分布于低潮位或潮下位边缘的类群未被充分记录。
3.3 优势种对群落结构的调节在青岛岩相潮间带,高潮带因环境恶劣,仅有粒结节滨螺和短滨螺等耐受性强的物种形成了优势种。此类环境限制了多数物种的生存,导致高潮带内物种间生态位重叠较少,群落结构主要通过生态位的垂直分化得以维持。中潮带则以东方小藤壶为优势物种,其强烈的种间竞争塑造了中潮带的群落结构。藤壶通过快速附着与密集生长,直接排斥了紫贻贝、长牡蛎等生态位相近的物种;另一方面,藤壶死亡后遗留的钙质壳体则形成了异质性微生境,又为短滨螺等物种的幼体提供了庇护场所,从而在局部尺度上维持并促进了生物多样性。需要注意的是,藤壶等固着生物在自然岩面上常呈高度聚集的斑块状分布,样方内个体数变异极大。本研究基于出现频率计算优势度,对这类分布极不均匀的物种可能会低估其实际的覆盖面积和生物量优势。未来研究中应结合覆盖度或生物量等多维度指标,进一步校准岩相潮间带藤壶类群优势程度的评估。
与青岛岩相潮间带历史调查结果相比,中潮位附近优势种组成表现出明显变化(见表 6)。二十世纪五六十年代,该区域以褶牡蛎(Ostrea plicatula)为绝对优势种[5-6];随后数十年间,紫贻贝逐步取代褶牡蛎成为主导类群[40-41]。本研究记录到东方小藤壶在此生境中形成数量优势,同时长牡蛎在部分潮位占优势,说明该区域固着性优势种组成正在发生新的变化。在温带地区平均气温升高,温度波动加剧的背景下,原有优势种(如紫贻贝)的耐受范围可能低于当下环境条件[45],而东方小藤壶和长牡蛎可能更适应这样严酷的气候变化。该机制与既有生理生态研究[37]及经典竞争模型[46]相吻合,也符合多个地区对藤壶分布区随气候与水动力条件而变化的观测结果[47-48]。
|
|
表 6 青岛岩相潮间带大型底栖动物优势种历史变化 Table 6 Historical changes in dominant macrobenthic species in Qingdao rocky intertidal zones |
温度是驱动群落结构变化的主要环境因子,而盐度、降水量和叶绿素a浓度等同样发挥了重要调节作用。这些环境因子通过影响物种的代谢过程、渗透调节和能量分配等生理机制,共同调控物种的生长、繁殖和分布,从而塑造了潮间带群落的垂直分布格局和季节性动态变化[49-50]。在暖季,较高的环境温度可能提高了腹足类物种(如马蹄螺目、新腹足目)的代谢速率和摄食效率,进而通过促进生长和繁殖提升其种群密度[51]。然而,这种促进作用具有季节性,随着温度下降,腹足类的代谢活动减缓,生长和繁殖速度下降,种群数量趋于稳定[52]。在冷季,低温环境促使暖季优势种(如腹足纲和多板纲)进入滞育或低活动状态[53],同时为耐寒性较强的物种(如长牡蛎和短滨螺)提供了有利条件。这些物种凭借较强的耐寒能力,在低温环境下维持种群稳定[51]。
4 结语本研究基于12个月的连续月度调查,系统揭示了青岛汇泉角岩相潮间带大型底栖动物群落的动态变化规律、纵向分布格局及其对环境因子的响应机制。与历史资料对比,群落优势种可能正在发生更替,东方小藤壶和牡蛎有一定取代传统优势类群的趋势。然而,本研究采样范围未涵盖低潮位和潮下带区域,可能导致部分物种的丰度被低估,从而影响对群落全貌的刻画。后续研究应拓展采样深度至潮下带,并结合长期连续监测,以更全面评估群落结构的时空变化趋势。
| [1] |
Mislan K S, Wethey D S, Helmuth B. When to worry about the weather: Role of tidal cycle in determining patterns of risk in intertidal ecosystems[J]. Global Change Biology, 2009, 15(12): 3056-3065. DOI:10.1111/j.1365-2486.2009.01936.x (  0) |
| [2] |
Kunze C, WÖlfelschneider M, RÖlfer L. Multiple driver impacts on rocky intertidal systems: The need for an integrated approach[J]. Frontiers in Marine Science, 2021, 8: 667168. DOI:10.3389/fmars.2021.667168 ( 0) |
| [3] |
Thyrring J, Peck L S. Global gradients in intertidal species richness and functional groups[J]. eLife, 2021, 10: e64541. DOI:10.7554/eLife.64541 ( 0) |
| [4] |
雷志远, 张明伟, 石鹏, 等. 青岛近岸海域大型底栖动物群落特征与底栖生态质量评价[J]. 中国海洋大学学报(自然科学版), 2025, 55(5): 87-99. Lei Z Y, Zhang M W, Shi P, et al. Macrobenthic community characteristics and benthic ecological quality assessment in the nearshore waters of Qingdao[J]. Periodical of Ocean University of China, 2025, 55(5): 87-99. DOI:10.16441/j.cnki.hdxb.20230161 ( 0) |
| [5] |
张玺. 《胶州湾海产动物采集团第一期采集报告》[M]. 北平(北京): 国立北平研究院出版课, 1935. Zhang X. First Collection Report of the Marine Animal Collecting Team in Jiaozhou Bay[M]. Beiping (Beijing): Publishing Section of the National Peiping Research Institute, 1935. ( 0) |
| [6] |
范振刚. 胶州湾潮间带生态学的研究——1.岩石岸潮间带[J]. 生态学报, 1981, 1(2): 117-125. Fan Z G. Studies on the intertidal ecology ofJiaozhou Bay-1. Rocky shore intertidal zone[J]. Acta Ecologica Sinica, 1981, 1(2): 117-125. ( 0) |
| [7] |
原大山, 刘志鸿, 马培振, 等. 青岛典型潮间带贝类的种类组成与群落特征[J]. 渔业科学进展, 2025, 46(1): 15-29. Yuan D S, Liu Z H, Ma P Z, et al. Species composition and community characteristics of mollusks in typical intertidal zones of Qingdao[J]. Progress in Fishery Sciences, 2025, 46(1): 15-29. ( 0) |
| [8] |
青岛市史志办公室. 青岛市志·自然地理志/气象志[M]. 北京: 新华出版社, 1997. Qingdao Municipal Local Chronicles Office. Qingdao Gazetteer: Natural Geography/Meteorology[M]. Beijing: Xinhua Publishing House, 1997. ( 0) |
| [9] |
Multi-Agency Rocky Intertidal Network (MARINe). MARINe/PISCO: Intertidal: MARINe Coastal Biodiversity Surveys: Coastal Biodiversity Survey Protocols[R]. [S. l. ]: PISCO MN, 2023.
( 0) |
| [10] |
John M E, Laura A, Jennifer L B, et al. Unified Monitoring Protocols for the Multi-Agency Rocky Intertidal Network[R]. Camarillo: Department of the Interior, Bureau of Ocean Energy Management, Pacific OCS Region, 2022.
( 0) |
| [11] |
王伟. 环境变化对我国岩相潮间带大型底栖生物地理格局的影响[D]. 厦门: 厦门大学, 2019. Wang W. TheImpacts of Environmental Change on the Biogeographic Patterns of Rocky Shore Macrobenthos Along China's Coast[D]. Xiamen: Xiamen University, 2019. ( 0) |
| [12] |
李新正, 王洪法. 胶州湾大型底栖生物鉴定图谱[M]. 北京: 科学出版社, 2016. Li X Z, Wang H F. Jiaozhou Bay Large Benthic Organism Identification Atlas[M]. Beijing: Science Press, 2016. ( 0) |
| [13] |
郑小东, 曲学存, 曾晓起, 等. 中国水生贝类图谱[M]. 青岛: 青岛出版社, 2013. Zheng X D, Qu X C, Zeng X Q, et al. Atlas of ChineseAquatic Mollusks[M]. Qingdao: Qingdao Publishing House, 2013. ( 0) |
| [14] |
李新正, 甘志彬. 中国近海底栖动物分类体系[M]. 北京: 科学出版社, 2022. Li X Z, Gan Z B. Classification System of Benthic Animals in China's Coastal Waters[M]. Beijing: Science Press, 2022. ( 0) |
| [15] |
WoRMS Editorial Board. World Register of Marine Species[EB/OL]. (2024-11-07)[2025-09-01]. https://www.marinespecies.org.
( 0) |
| [16] |
Hersbach H, Bell B, Berrisford P, et al. ERA5 hourly data on single levels from 1940 to present[EB/OL]. (2018-06-14)[2024-12-11]. https://doi.org/10.24381/cds.adbb2d47.
( 0) |
| [17] |
Copernicus. Global Ocean Physics Analysis and Forecast[EB/OL]. (2024-12-11)[2025-09-01]. https://doi.org/10.48670/moi-00016.
( 0) |
| [18] |
Copernicus M S I (CMEMS). Global Ocean Biogeochemistry-Analysis and Forecast[EB/OL]. (2024-12-11)[2025-09-01]. https://doi.org/10.48670/moi-00281.
( 0) |
| [19] |
Mcnaughton S J. Relationships among functional properties of Californian Grassland[J]. Nature, 1967, 216(5111): 168-169. ( 0) |
| [20] |
Strong W L. Biased richness and evenness relationships within Shannon-Wiener index values[J]. Ecological Indicators, 2016, 67: 703-713. DOI:10.1016/j.ecolind.2016.03.043 ( 0) |
| [21] |
Ricotta C, Avena G. On the relationship between Pielou's evenness and landscape dominance within the context of Hill's diversity profiles[J]. Ecological Indicators, 2003, 2(4): 361-365. DOI:10.1016/S1470-160X(03)00005-0 ( 0) |
| [22] |
Margalef R. Perspectives in Ecological Theory[M]. Chicago, London: University of Chicago Press, 1968.
( 0) |
| [23] |
Wickham H. Ggplot2:Elegant Graphics for Data Analysis[M]. 2nd ed. Cham: Springer Cham, 2016.
( 0) |
| [24] |
Tiedemann F. Gghalves: Compose Half-Half Plots Using Your Favourite Geoms[CP/OL]. (2022-11-20)[2025-08-21]. https://cran.r-project.org/web/packages/gghalves/index.html.
( 0) |
| [25] |
Rosa J, Muniz C M, Petsch D K, et al. Local factors drive the richness, biomass and composition of benthic invertebrate communities in Neotropical reservoirs[J]. Aquatic Sciences, 2024, 86(2): 61. DOI:10.1007/s00027-024-01064-z ( 0) |
| [26] |
Oksanen J, Simpson G L, Blanchet F G, et al. Vegan: Community ecology package[R]. Vienna: Comprehensive R Archive Network, 2026.
( 0) |
| [27] |
Borg I. Data fit (stress) vs model fit (recovery) in multidimensional scaling[J]. Austrian Journal of Statistics, 2020, 49(2): 43-52. DOI:10.17713/ajs.v49i2.918 ( 0) |
| [28] |
Clarke K, Ainsworth M. A method of linking multivariate community structure to environmental variables[J]. Marine Ecology Progress Series, 1993, 92: 205-219. DOI:10.3354/meps092205 ( 0) |
| [29] |
Liu C, Cui Y, Li X, et al. Microeco: An R package for data mining in microbial community ecology[J]. FEMS Microbiology Ecology, 2021, 97(2): 255. DOI:10.1093/femsec/fiaa255 ( 0) |
| [30] |
Reiss H, Meybohm K, Kröncke I. Cold winter effects on benthic macrofauna communities in near-and offshore regions of the North Sea[J]. Helgoland Marine Research, 2006, 60: 224-238. DOI:10.1007/s10152-006-0038-3 ( 0) |
| [31] |
Chen N, Liu Y, Yuan L, et al. Adaptive mechanisms of invasion of Chthamalus challengeri (Hoek, 1883) in the trans-oceanic zone of coastal China[J]. Aquatic Invasions, 2024, 19(1): 1-23. DOI:10.3391/ai.2024.19.1.115111 ( 0) |
| [32] |
Ubertini M, Lagarde F, Mortreux S, et al. Gametogenesis, spawning behavior and larval abundance of the Pacific oyster Crassostrea gigas in the Thau lagoon: Evidence of an environment-dependent strategy[J]. Aquaculture, 2017, 473: 51-61. DOI:10.1016/j.aquaculture.2017.01.025 ( 0) |
| [33] |
Montes A, Vázquez E, Peteiro L, et al. Dynamics and processes influencing recruitment of the invasive mussel Xenostrobus securis and the coexisting indigenous Mytilus galloprovincialis in north-western Spain[J]. Aquatic Invasions, 2021, 16(3): 391-414. DOI:10.3391/ai.2021.16.3.02 ( 0) |
| [34] |
Thomas Y, Bacher C. Assessing the sensitivity of bivalve populations to global warming using an individual-based modelling approach[J]. Global Change Biology, 2018, 24(10): 4581-4597. DOI:10.1111/gcb.14402 ( 0) |
| [35] |
Lu X, Xu J, Xu Z, et al. Assessment of benthic ecological quality status using multi-biotic indices based on macrofaunal assemblages in a Semi-Enclosed Bay[J]. Frontiers in Marine Science, 2021, 8: 734710. DOI:10.3389/fmars.2021.734710 ( 0) |
| [36] |
杨万喜, 陈永寿. 嵊泗列岛潮间带群落生态学研究Ⅰ.岩相潮间带底栖生物群落组成及季节变化[J]. 应用生态学报, 1996, 7(3): 305-309. Yang W X, Chen Y S. Community ecology of the intertidal zone in the Shengsi Archipelago Ⅰ: Composition and seasonal variation of benthic communities in the rocky intertidal zone[J]. Chinese Journal of Applied Ecology, 1996, 7(3): 305-309. ( 0) |
| [37] |
Chiba S, Iida T, Tomioka A, et al. Population divergence in cold tolerance of the intertidal gastropod Littorina brevicula explained by habitat-specific lowest air temperature[J]. Journal of Experimental Marine Biology and Ecology, 2016, 481: 49-56. DOI:10.1016/j.jembe.2016.04.009 ( 0) |
| [38] |
Takada Y. Seasonal andlong-term fluctuations in a population of Patelloida heroldi (Mollusca: Gastropoda) on a boulder shore in Japan[J]. VENUS, 2007, 66(1-2): 85-97. ( 0) |
| [39] |
Villarta K A. Life History Strategies of the Limpet Cellana toreuma and Its Physiological Response to Environmental Stress[D]. Hong Kong: University of Hong Kong, 2015.
( 0) |
| [40] |
唐贵明, 钟瑜, 曾晓起. 青岛岩相潮间带大型底栖动物生物多样性调查研究[J]. 南方水产, 2008, 4(5): 8-15. Tang G M, Zhong Y, Zeng X Q. Study on biodiversity of macrobenthic fauna in the rocky intertidal zone of Qingdao[J]. South China Fisheries Science, 2008, 4(5): 8-15. ( 0) |
| [41] |
姚韡远. 青岛近岸与大公岛岩礁区大型底栖生物群落研究[D]. 青岛: 中国海洋大学, 2014. Yao W Y. Study on Macrobenthic Communities in the Nearshore of Qingdao and the Rocky Reef Area of Dagong Island[D]. Qingdao: Ocean University of China, 2014. ( 0) |
| [42] |
Shou L, Liao Y, Tang Y, et al. Seasonal distribution of macrobenthos and its relationship with environmental factors in Yellow Sea and East China Sea[J]. Journal of Oceanology and Limnology, 2018, 36(3): 772-782. DOI:10.1007/s00343-018-6271-1 ( 0) |
| [43] |
韩庆喜, 袁泽轶, 陈丙见, 等. 烟台潮间带大型底栖动物群落组成和结构研究[J]. 海洋科学, 2014, 38(9): 59-68. Han Q X, Yuan Z Y, Chen B J, et al. Community composition and structure of macrobenthos in Yantai intertidal zone[J]. Marine Sciences, 2014, 38(9): 59-68. ( 0) |
| [44] |
刘东艳, 韩秋影. 潮间带调查方法与实践[M]. 北京: 科学出版社, 2016. Liu D Y, Han Q Y. Intertidal Survey Methods and Practice[M]. Beijing: Science Press, 2016. ( 0) |
| [45] |
韩国栋. 典型潮间带贝类温度生理适应及其分子机制[D]. 厦门: 厦门大学, 2018. Han G D. Physiological Adaptation of Typical Intertidal Molluscs to Thermal Stress[D]. Xiamen: Xiamen University. 2018. ( 0) |
| [46] |
Connell J H. The influence of interspecific competition and other factors on the distribution of the barnacle Chthamalus stellatus[J]. Ecology, 1961, 42(4): 710-723. DOI:10.2307/1933500 ( 0) |
| [47] |
Wares J P. Small, flat, and gray: Cryptic diversity in chthamalid barnacles in the global context of marine coastal biogeography (Cirripedia: Balanomorpha: Chthamalidae)[J]. Journal of Crustacean Biology, 2019, 40(1): 1-16. ( 0) |
| [48] |
Wethey D S. Geographic limits and local zonation: The barnacles Semibalanus (Balanus) and Chthamalus in New England[J]. Biological Bulletin, 1983, 198: 330-341. ( 0) |
| [49] |
Sokolova I M, Frederich M, Bagwe R, et al. Energy homeostasis as an integrative tool for assessing limits of environmental stress tolerance in aquatic invertebrates[J]. Marine Environmental Research, 2012, 79: 1-15. ( 0) |
| [50] |
Kültz D. Physiological mechanisms used by fish to cope with salinity stress[J]. Journal of Experimental Biology, 2015, 218(12): 1907-1914. DOI:10.1242/jeb.118695 ( 0) |
| [51] |
Dong Y W. Roles of multi-level temperature-adaptive responses and microhabitat variation in establishing distributions of intertidal species[J]. Journal of Experimental Biology, 2023, 226(21): 245745. DOI:10.1242/jeb.245745 ( 0) |
| [52] |
Stickle W B, Carrington E, Hayford H. Seasonal changes in the thermal regime and gastropod tolerance to temperature and desiccation stress in the rocky intertidal zone[J]. Journal of Experimental Marine Biology and Ecology, 2017, 488: 83-91. DOI:10.1016/j.jembe.2016.12.006 ( 0) |
| [53] |
Reid H B, Harley C D G. Low temperature exposure determines performance and thermal microhabitat use in an intertidal gastropod (Littorina scutulata) during the winter[J]. Marine Ecology Progress Series, 2021, 660: 105-118. DOI:10.3354/meps13588 ( 0) |
2. Shandong Key Laboratory of Green Mariculture and Smart Fishery, Ocean University of China, Qingdao 266003, China;
3. Academy of Future Ocean, Ocean University of China, Qingdao 266100, China